A Whiff of Taxonomy – Cycloclasticus
(And a Whiff of Symbiosis)
by Christoph
Whenever you stumble across the name of a bacterial species you've never heard of before you probably wonder what the heck that name wants to tell you. Sure, you are likely familiar with the venerable tradition in all of biology to name species according to the rules outlined by Linnaeus: a genus name followed by a species name, both names in Latin (with a pinch of ancient Greek), or at least sounding latin-ish (here's a phonetic pronunciation guide for English speakers that makes people shudder who have more-than-basic knowledge of Latin and its pronunciation). As a native English speaker, wouldn't you just smile and guess that the species name Gynuella sunshinyii is a tongue-in-cheek parody of Linnaeus' rules? Not so. This Gammaproteobacterium of the order Oceanospirillales was actually named after Sun Shin Yi, a renowned Korean naval commander of the 15th century, who died during a battle at Namhae Island, where the type strain was isolated. And the genus name Gynuella refers to Gyeongsang National University, Jinju, South Korea (you can "locate" the Oceanospirillales in Figure 2).

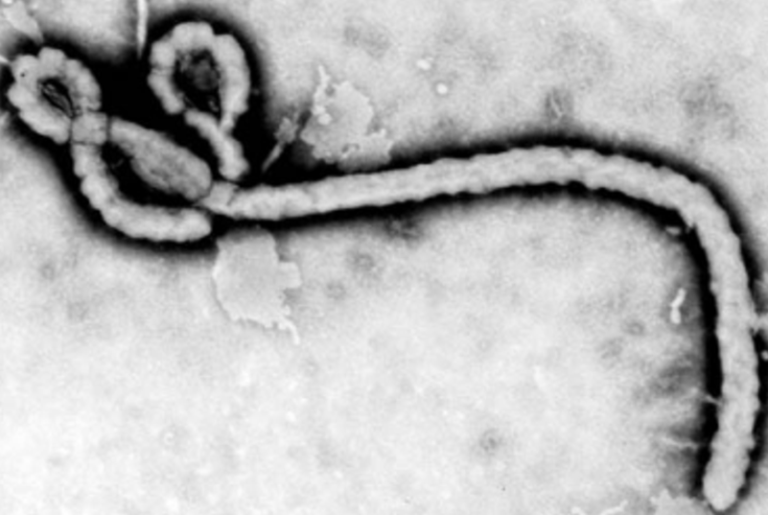
Figure 1. FISH images of Cycloclasticus endosymbionts. a Patches of Cycloclasticus (green) in B. heckerae gill filaments that also host methanotrophic symbionts (red). Bar = 20 µm. b Intracellular Cycloclasticus symbionts (green) co-occur with the larger methanotrophic symbionts (red) intracellularly in bacteriocytes of B. heckerae gill tissues. Bar = 5 µm. Click here to see b. Source. Frontispiece: Negatively stained preparation of a Cycloclasticus pugetii PS‑1T cell showing the single polar flagellum and numerous fimbriae sticking out from the cell surface. Bar = 200 nm. Bar = 200 nm. Source
Having said this, you probably hesitate to think of ancient Roman circus games and gladiators when I now introduce Cycloclasticus. Rightly so, the dramatic-sounding name translates to "the one who breaks rings into pieces" and refers to the remarkable property of several species of this bacterial genus to break down and make a living on polycyclic aromatic hydrocarbons (PAHs).
Cycloclasticus pugetii, the first fully characterized member of the genus, was isolated in 1991 from creosote-contaminated sediment samples (16°C, 32% salinity) collected at three different sites of the Puget Sound. C. pugetii cells grow aerobically in synthetic media that mimic seawater. They are catalase-positive, oxidase-positive, reduce nitrate to nitrite, and are motile rods of 0.5 by 1.0 – 2.0 µm, adorned with numerous fimbriae and a single polar flagellum (see frontispiece). Metabolic profiling tells us that they do not grow on one-carbon compounds, simple hydrocarbons (ethanol, hexadecane), organic acids, amino acids, intermediates (α‑ketoglutarate, pyruvate, butyrate), and carbohydrates. They grow, however, on carbon compounds like biphenyl, naphthalene, anthracene, phenanthrene – all four being PAHs – salicylate, toluene, benzoate, acetate, propionate, and glutamate, at temperatures from 4 – 28°C, in salinities ranging from 10 – 70%, and at pH values ranging from 6.5 to 9.5.

Figure 2. Phylogenetic tree of seafloor basalt Gammaproteobacteria based on the hypervariable V4 region of the 16S rRNA gene. Tree topology determined using publicly available nearly full-length sequences from environmental samples or cultivated representatives (GenBank accession number in parentheses), with representatives of shorter tag OTUs from this study inserted with pplacer. Closely related OTUs from this study are grouped together into fans, with number of Dorado tag OTUs indicated in parentheses followed by number of sequences from all rock samples (n=13), and bottom seawater samples (n=2). Sequences from other seafloor basalt samples that group most closely to OTU fans indicated by symbols shown in legend. Support for branching patterns of the maximum likelihood tree from 1000 bootstraps reported at the nodes. Mariprofundus ferrooxydans (Zetaproteobacteria) was used as the outgroup (not shown). Note that "Salinocola socius (DQ979342)" in the Oceanospirillales cluster should read as Salinicola socius (DQ979342). The position of Cycloclasticus is indicated by a red arrow. Source
In 1995, Dyksterhouse et al. concluded from 16S rRNA sequencing that C. pugetii belongs to the Gammaproteobacteria but a more precise assignment to one of the various taxonomic orders or families was impossible at that time. If you think of Gammaproteobacteria, you're familiar, of course, with Escherichia coli and other Enterobacterales – the former Enterobacteriales have lost their "i" in the meantime – like Salmonella, Yersinia X, Serratia X, and Sodalis X. You are likely well aware of Vibrio cholerae X from the Vibrionales, a sister order of the Enterobacterales. And you can hardly have missed STC's frequent mentioning of Pseudomonas X and its ilk. But there are many more that we mentioned as "...from the Gammaproteobacteria" without taking much care to indicate their position in the gammaproteobacterial "tree": Xylella fastidiosa X (Xanthomonadales), Acinetobacter baumannii X (Moraxellaceae), Thioploca chileae X and Thiomargarita X (Thiotrichales), Francisella tularensis X (Francisellaceae), Coxiella burnetii X (Legionellales), Profundimonas piezophila X (Oceanospirillales), to name a few. You find most of them in a paper from 2010, 'Phylogeny of Gammaproteobacteria' by Williams et al., and therein in the lower part of their tree (Figure 3, here) lumped together in a cluster "Basal", which is by no means a valid taxonomic category. We're better off today thanks to coordinated efforts to sequence ~11,000 genomes across the entire bacterial and archaeal domains and extensive metagenomic sampling. It is thus no longer difficult to "find" Cycloclasticus in its proper phylogenomic context, for example in the tree of seafloor basalt Gammaproteobacteria assembled by Beth Orcutt and her collaborators at the Bigelow Laboratory for Ocean Sciences from reference genomes, their own data, and related studies by other marine microbial biogeochemists (red arrow in Figure 2). The "basal" groups of Williams et al. are now nicely dissected – with only few murky overlaps – in this survey of basal-t-dwelling Gammaproteobacteria (irresistible pun), and Cycloclasticus clearly clusters (irresistible alliteration) with other Thiotrichales, which in turn are well separated from the Chromatiales and Oceanospirillales. Missing from their tree are the Xanthomonadales that weren't present in their samples taken at 3,000 m below the sea surface from basaltic rock at the Dorado Outcrop, a site of low-temperature hydrothermal venting (<20°C) on the eastern flank of the East Pacific Rise. This site revealed much greater richness and diversity on these floor rocks than in surrounding seawater but you probably miss the Vibrionales and Enterobacterales in the tree. If they were included in Figure 2, they would branch-off from the Alteromonadales next to Shewanella, just as can be seen in the Williams et al. tree. Although the tree shown in Figure 2 does not indicate the abundance of individual Gammaproteobacteria, the presence of almost all orders of the Gammaproteobacteria at the sample sites strongly reminds me on the Baas-Becking hypothesis "Everything is everywhere, but the environment selects".
Now, a Whiff of Symbiosis...
Ten years ago, our (by now) emerita Merry introduced deep sea mussels to this blog, mainly considering their small-thingy symbionts that were known since 1988. She wrote: "Certain mussels called "bathymodiolins" are part of the spellbinding fauna of the dark world of oceanic hydrothermal vents and cold seeps. Similar to other metazoans in that realm, they rely on chemosynthetic bacteria for their nutrition. These mussels possess symbionts from two clades of γ‑proteobacteria: chemoautotrophic sulfur oxidizers that fix CO2 using sulfide or thiosulfate as their energy source, and methane oxidizers that use methane for both carbon and energy. The symbionts are well-housed in specialized cells (bacteriocytes) in the gills of the mussels where the constant flow of water brings the needed substrates to them. A pleasant mutualistic arrangement." Merry's post also referred to work from Nicole Dubilier's lab at the MPI for Marine Microbiology in Bremen, Germany, on a intranuclear bacterial parasite of bathymodiolins, Candidatus Endonucleobacter bathymodioli (Oceanospirillales), and I will follow here with featuring a more recent study from this lab on yet another symbiont of Bathymodiolus heckerae mussels and poecilosclerid sponges, Cycloclasticus of course, you guessed it.

Figure 3. MARUM-Quest ROV image of symbiont-bearing fauna at Chapopote seepage hotspot. Bathymodiolus heckerae, B. brooksi (undistinguishable from B. heckerae in the image), encrusting and branching sponges were collected. Source
Rubin‑Blum et al. collected mussels and sponges with a ROV during their 2015 research cruise to the Campeche Knolls in the southern Gulf of Mexico, where lava-like flows of solidified asphalt, oil seeps, gas hydrate deposits, and locally anoxic sediments cover roughly 50 km2 of the rim of a dissected salt dome at a depth of 3,000 m. Sample collection took place at two locations, the Chapopote "bubble" site (21°54' N; 93°26' W) with flourishing faunal communities in the presence of fresh asphalts and exposed gas hydrates (Figure 3), and the Mictlan Knolls site (22°1' N; 93°14' W) with considerable gas and oil bubbling. The symbiont-bearing gills of the mussels and the sponge tissues were dissected and fixed immediately after retrieval for FISH analysis with probes targeting Cycloclasticus – first detected at the same site during an earlier study in 2006 – and the methanotrophic/thiotrophic symbionts. The presence of Cycloclasticus endosymbionts was confirmed for the eight collected B. heckerae mussels and all three collected sponge species but they were missing from the gills of the four B. brooksi mussels (Figures 1 + 4). Since Cycloclasticus are distributed in small patches among the other symbionts in the FISH analysis of gill tissue (Figure 1), they 'counted' metagenomic sequence reads for all samples that mapped to Cycloclasticus 16S rRNA and can thus estimate that the relative abundance of Cycloclasticus is approximately 5 – 11% of all mussel symbionts, and 4 – 8% of the sponge symbionts.
Phylogenetic analyses of the Cycloclasticus 16S rRNA gene sequences from the Campeche Knoll B. heckerae mussels and sponges revealed that they were phylogenetically distinct from each other but belong to a closely-related clade (98% similarity) of cultivated and environmental Cycloclasticus found earlier in oil-contaminated environments as, for example, the Deepwater Horizon oil spill. They were, however, phylogenetically distinct from cultivated Cycloclasticus, such as C. pugetii. Since B. heckerae and the two sponge species each harbor a specific Cycloclasticus 16S rRNA phylotype that differs between these three host species but is nearly identical (>99%) between individuals of the same host species from the two collection sites Chapopote and Mictlan, separated by 25 km, Rubin-Blum et al. think it appropriate to use the term 'symbiotic' for these host-specific bacteria. The FISH analyses show clearly that the Cycloclasticus symbionts thrive intracellularly in the mussel gills and sponge tissue, they are thus endosymbionts. However, it is presently unknown whether they are transmitted maternally, that is, vertically, or horizontally (which seems more likely).

Figure 4. FISH images of Cycloclasticus endosymbionts. d High-res image of Cycloclasticus within the encrusting sponge tissues (3D reconstruction from 2D z‑stacks). Bar = 5 µm. Source
The researchers assembled Cycloclasticus draft genomes (93 – 97% complete) from the metagenomic sequencing of four B. heckerae individuals sampled at the Chapopote site, which have estimated sizes of 2.1 – 2.2 Mb and an average nucleotide identity (ANI) of ≥ 99.95%. The Cycloclasticus draft genomes (93 – 97% complete) from the two encrusting sponge species have estimated sizes of 1.6 – 2.3 Mb and, again, are highly similar to each other (ANI = 99.8%) despite the fact that these hosts were collected at two sites separated by 20 km. These genomes differ markedly from the Cycloclasticus genome of the branching sponge (ANI = 79.8%) and the B. heckerae mussels (ANI values below 80%). ANI values, phylogenetic 16S rRNA, and additional phylogenomic analyses support the conclusion that the three invertebrate species examined by Rubin-Blum et al. here harbor highly host-specific Cycloclasticus symbionts. And, noteworthy, all symbiont genomes are a tad smaller than those of cultivated Cycloclasticus species (2.4 – 3.65 Mb).
In incubation experiments with Cycloclasticus-bearing B. heckerae gill tissues, they did not observe oxidation of 14C‑labelled naphthalene to 14CO2, while control experiments with C. pugetii showed the expected naphthalene oxidation. And indeed, close inspection of the genomes of the Cycloclasticus symbionts revealed that they all lack genes involved in PAH degradation. Neither were PAH degradation-specific genes/transcripts and proteins detected in the metagenomic, metatranscriptomic and metaproteomic data (whole sample data, that is, from all symbionts and the respective host). Instead, Rubin-Blum et al. found high expression levels of genes involved in the use of short-chain alkanes. Therefore, the symbiotic Cycloclasticus most likely use gaseous non-aromatic short-chain hydrocarbons as energy and carbon sources. They had measured the concentrations and relative proportions of short-chain alkanes in the environment of the symbiont-bearing invertebrates by sampling and analyzing gas and oil bubbles a few centimeters above the collection sites at Chapopote and Mictlan, and a piece of surface asphalt with gas hydrate from the immediate vicinity of mussels and sponges at Chapopote. Concentrations of ethane, propane and butane in the asphalt were in the micromolar (µM) to low millimolar (mM) range, and thus sufficiently high to feed the Cycloclasticus symbionts. Taken together, these findings were surprising, as all cultivated Cycloclasticus are able to degrade PAH, but do not appear to use short-chain alkanes. In contrast to the genomes of the symbiotic Cycloclasticus, the genomes of cultivated Cycloclasticus lack genes coding for the first two enzymes needed for short-chain alkane oxidation, hydrocarbon monooxygenases (pHMOs) and alcohol dehydrogenases (PQQ-ADHs). Aldehyde ferredoxin oxidoreductases (AORs), the third group of enzymes, are present in the genomes of cultivated Cycloclasticus but their protein sequences are only 70% similar to those of the symbiotic Cycloclasticus. It is remarkable to find such metabolic variability within the clade of closely related Cycloclasticus species with >98% 16S rRNA identity.
Call it an 'encore', but there is something else that can be learned from the research on Cycloclasticus described here, something that's more at the meta level. When the lab of James T. Staley at the University of Washington, Seattle, WA, isolated Cycloclasticus pugetii, they studied its metabolic properties in vivo, that is by growth tests on a battery of different carbon compounds (see 2nd paragraph). Such growth tests can generate, when performed as a combinational ballet, virtually complete metabolic profiles for the studied species. The same researchers found, by one such "ballet", that Neptunomonas naphthovorans NAG-2N-113 (Oceanospirillales), another isolate from creosote-contaminated sediment from the Puget Sound, degrades 2,6‑dimethylnaphthalene and phenanthrene, but acenaphthene was only degraded in a mixture of seven other PAHs. Enter the biochemists who identify the proteins that perform the required enzymatic reactions in vitro, and the geneticists who identify the genes for a metabolic pathway and its regulation. That's the 'classical' top-down approach. Rubin-Blum et al. could not grow their Cycloclasticus symbionts in the lab, for obvious reasons, but "sequenced them", that is both their genomes and their transcriptomes, and assessed their proteomes via mass-spectrometry. They could thus reconstruct the symbionts' metabolic capacities in silico by homology searches for genes/proteins with known functions (see here for their in silico metabolic profiles ). That's the bottom-up approach, much en vogue today. The two approaches are not mutually exclusive, quite the contrary, they complement each other. While the bottom-up approach crucially depends on the 'treasure trove' of functionally characterized gene sequences in the data bases obtained by the top-down approach, the latter gets an hefty update of its list of not-yet-asked questions with every newly completed genome sequencing project. Even after complete sequencing of ~6,300 prokaryotic genomes, roughly 1/3 of all genes in normal sized bacterial and archaeal genomes (3 – 5 Mb) cannot be assigned a function. Fun fact: the synthetic 531,560 bp-long chromosome of the Mycoplasma derivative JCVI-syn3.0 contains 473 genes, 149 of which whose functions are completely unknown.